N-Glycosylation in Cell-Free Protein Synthesis Systems
Researchers overcome timing barriers to add glycans during cell-free protein synthesis.
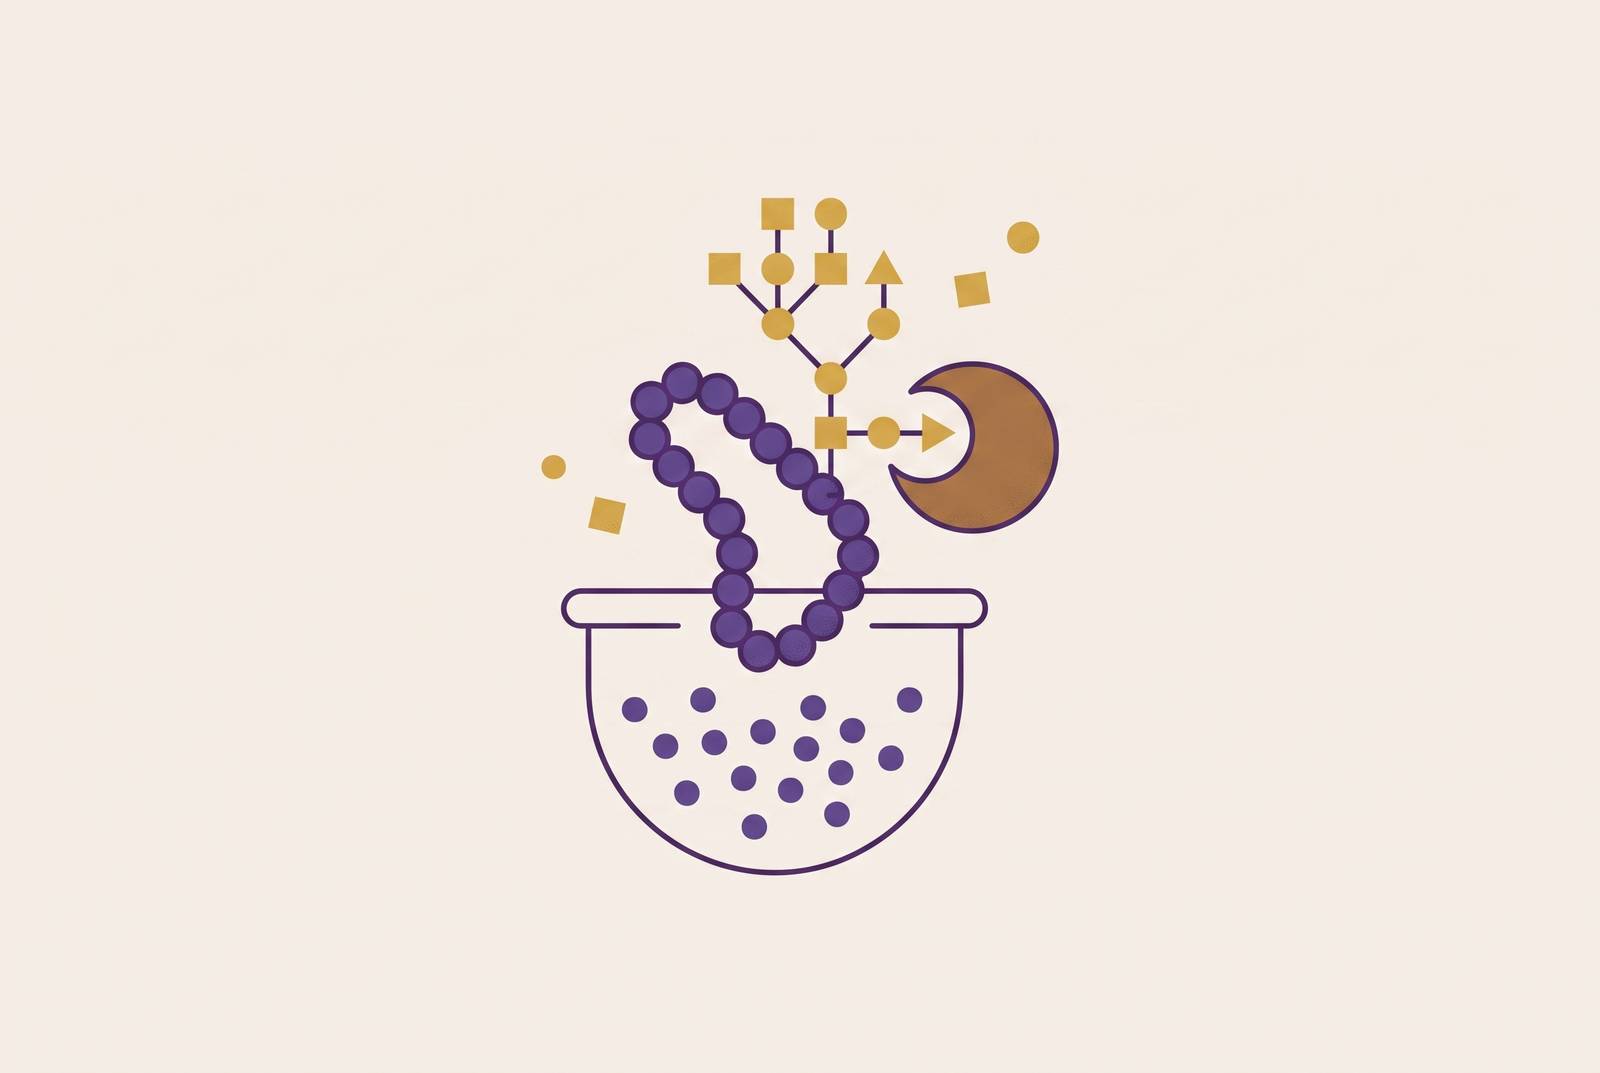
N-glycosylation is still a major unsolved challenge in cell-free protein synthesis (CFPS) because glycan transfer depends on the protein’s structure and the timing as well as which enzymes are available. Strategies designed for this task can preserve co-translational access or work around its loss. Their usefulness depends on two separate requirements, namely whether the target site remains accessible and whether the installed glycan meets the application’s needs.
Why N-glycosylation is the hardest PTM for cell-free systems to replicate
N-glycosylation depends on cellular architecture that most CFPS platforms remove. In eukaryotic cells, the nascent polypeptide passes through the Sec61 translocon into the endoplasmic reticulum (ER) lumen. There, the oligosaccharyltransferase (OST) complex recognises an N-X-S/T sequon and transfers a pre-assembled oligosaccharide from a dolichol-linked precursor onto asparagine before the domain folds. Timing is part of the mechanism itself. LenioBio’s 2026 characterisation describes this co-translational process and its consequences for cell-free platform design.
Standard E. coli extracts lack glycosylation machinery entirely, while rabbit reticulocyte and wheat germ extracts lack functional microsomes and require exogenous microsomal membranes for native N-glycosylation. Architectural deficits that persist after simple supplementation restrict applications involving proteins such as IgG Fc and erythropoietin, whose glycosylation supports functions including effector activity or serum half-life. Bidstrup et al.’s 2025 ACS Synthetic Biology study showed that structurally constrained acceptor sites in ribonuclease A and IgG Fc resisted glycosylation after folding. For these targets, solving glycosylation means solving co-translational coupling.
Why the OST machinery's timing requirement is the central design constraint engineers must work around
The OST requires access to a flexible acceptor segment. In nearly all bacterial N-linked glycosylation systems, a single-subunit transmembrane OST performs glycan transfer, exemplified by PglB from Campylobacter jejuni. It favours flexible, solvent-exposed substrate motifs over sites buried within folded domains. Consequently, a post-translational reaction cannot compensate for a sequon that has already become inaccessible.
CFPS exposes this constraint while providing ways to address it. Its open reaction environment gives direct control over what goes into the reaction and when, but removes the translocon, ER membrane and native OST orientation that normally link synthesis with glycan transfer. Access must therefore be preserved or engineered.
Two engineering philosophies respond to this shared constraint. Eukaryotic extracts retain or reconstitute ER-like microsomes so that the OST intercepts the nascent chain during synthesis. Prokaryotic approaches instead use engineered OST variants, separate expression from glycosylation, or target flexible regions that remain accessible after folding. These approaches are complementary rather than interchangeable, because an improvement in transfer activity does not necessarily overcome structural occlusion.
How prokaryotic CFPS extracts engineer around the glycosylation gap using PglB variants and pathway assembly
E. coli-based CFPS combines high volumetric yield and low reagent cost with a glycosylation gap that requires deliberate engineering. DeWinter et al.’s 2024 ACS Chemical Biology study established a cell-free system for enzymatic N-GlcNAcylation using extracts enriched with PglB^N311V. This mutant has greater GlcNAc transferase activity than wild-type PglB, and reaction optimisation achieved 98.6 ± 0.5% glycosylation efficiency. The product is a defined single-GlcNAc glycoform. That sugar provides a primer for downstream chemoenzymatic elaboration, but does not itself constitute a complex or oligomannose glycan.
GlycoPRIME addresses glycan diversity through modular pathway assembly. CFPS enriches crude lysates with glycosyltransferases, after which combinations of those lysates form different pathways and generate distinct glycan motifs on target proteins. This allows different combinations to be tested without living cells. It does not reproduce the native eukaryotic processing cascade of glucosidase trimming and Golgi elaboration, however, and multi-sugar construction requires the relevant additional enzymes.
Neither strategy reconstitutes the ER’s co-translational window, so site accessibility remains a boundary condition. A 2025 Nature Communications study described GlycoSCORES, which couples CFPS to SAMDI mass spectrometry for rapid functional screening of glycosyltransferase variants.
How the two-step decoupling strategy resolves the yield and glycosylation-efficiency tension in prokaryotic systems
The carrier protein is first expressed for yield, then exposed to PglB-mediated glycosylation in a controlled second reaction. Each stage can be optimised independently. This resolves a process trade-off while retaining the structural requirement for an accessible acceptor site, so it is suited to substrates that remain glycosylation-competent after synthesis.
Wong et al.’s 2025 preprint applied this architecture to conjugate vaccines targeting enterotoxigenic E. coli O78 and Streptococcus pneumoniae serotype 4. Earlier cell-free conjugate vaccine work used 15 µL reactions, relatively low protein yields and basic gravity-flow purification that produced low purity. The two-step platform achieved high glycosylation efficiency and substantially higher glycoprotein titers, completing production in under five days with high purity and low endotoxin levels suitable for preclinical evaluation. Immunisation of mice with the pneumococcal conjugate induced a strong IgG response against serotype 4 capsular polysaccharide, although these findings remain preprint evidence.
The installed glycans are bacterial-type or simplified, and further chemoenzymatic steps are needed to make complex human-type structures. Cell-free reactions can be lyophilised for long-term, non-refrigerated storage and reactivated at the point of use. That compatibility supports decentralised vaccine manufacturing in resource-limited settings without maintaining a living production culture at the destination.
How plant-cell eukaryotic extract retains native OST machinery and what that delivers and does not deliver
ALiCE® keeps the cell’s machinery in place. Developed by LenioBio GmbH from Nicotiana tabacum BY-2 cells, the extract retains intact ER and Golgi microsomes, native OST, glucosidases, SRP targeting machinery and the dolichol-linked precursor pool. Nascent proteins are trafficked to microsomes during synthesis. This preserves the co-translational window rather than relying on access to the completed protein.
LenioBio’s characterisation analysed three glycoproteins by LC-ESI-MS/MS across three independent lysate batches. Glucose oxidase had five detected N-glycosylation sites, N111, N280, N377, N410 and N495, with Man8 dominant at occupied sites and lower levels of Man7 and Man6. Hybrid and complex-type species were minimal. Adalimumab’s single CH2-domain site also showed a Man8-dominated spectrum, unlike the clinical CHO-produced complex-type biantennary glycoform with core fucosylation in the G0F/G1F/G2F series. SARS-CoV-2 RBD sites N331 and N343 were predominantly Man8, although N343 also showed hybrid-type and GnGn species.
These profiles were highly reproducible across lysate batches. They indicate partial Golgi processing, but most glycans did not complete the processing sequence of an intact secretory pathway. Native occupancy therefore does not imply mammalian-like maturation. The output is useful where high-mannose glycosylation is adequate, including many research reagents, vaccine antigens and enzymes requiring thermostability. Defined complex-type fucosylation or sialylation remains outside the platform’s current deliverable.
The platform also provides continuity between screening and production. It spans 96-well screening, 100 mL preparative reactions and 1,000 mL bioreactor production. The glycoform limitation remains at each scale, but the same platform can be used as reactions grow beyond screening volumes.
What the IgG Fc glycosylation result reveals about which targets each platform can and cannot serve
Bidstrup et al. demonstrated that an E. coli-based cell-free glycoprotein synthesis system could efficiently glycosylate human IgG Fc and RNase A when transfer was coupled co-translationally. Pre-folded substrates resisted the same intervention. This distinction prevents a misleading division between “glycosylating” and “non-glycosylating” extract types. A prokaryotic reaction can glycosylate a structured-domain target if transfer happens at the right time, even without recreating the ER.
For researchers choosing a platform, sequon accessibility is therefore the first decision axis. A flexible, surface-exposed loop can remain compatible with post-translational transfer and two-step processing, while a constrained site such as that in IgG Fc requires co-translational access. Glycoform identity is a separate requirement. Fc glycosylation governs FcγR binding, complement activation and antibody-dependent cellular cytotoxicity, so occupancy alone does not establish suitability for an antibody application.
Where oligomannose is acceptable, plant-cell extract provides native glycosylation with demonstrated batch reproducibility. For accessible bacterial glycan conjugation targets, two-step processing offers strong glycosylation efficiency at scale, while prokaryotic systems retain advantages in yield and reagent cost. Neither choice resolves every target requirement. No current CFPS platform fully replicates complex-type biantennary glycans with human-appropriate fucosylation and sialylation patterns, for which mammalian cell-based production remains the reference.
Toxic proteins, membrane proteins such as GPCRs and insoluble proteins benefit from an open environment that bypasses cellular viability constraints. Those advantages remain distinct from glycan capability.
How high-throughput glycoprotein screening and automation integration are changing what CFPS can do at scale
The same open environment that lets researchers control timing also lets them screen variants quickly. CFPS removes cloning, transformation, colony screening and culture optimisation steps between library design and glycosylation readout. GlycoSCORES exploits that separation through label-free, quantitative peptide glycosylation analysis using self-assembled monolayers for SAMDI mass spectrometry. The assay avoids time-consuming cell lysis and protein purification. The Nature Communications study screened hundreds of enzyme variants, identified a mutant with a 1.7-fold improvement in glycosylation using a clinically relevant glycan, and characterised accessible sites in a regulator-approved carrier protein.
A December 2025 preprint described how OT-2 liquid handling was used to assemble reconstituted cell-free systems from modules, with enough for 50 reactions at 25 µL scale. MANGO (MANufacturing on the GO) automates benchtop CFPS and purification through computer-controlled pumps, valves and a microchannel manifold. A 2025 preprint described its deployment in Brazil and Colombia for patient-trial diagnostics. These examples show which tasks can be automated, but leave open whether every automated configuration supports glycosylation.
Plate-based workflows fit standard incubators and liquid handlers. For glycoengineering, that compatibility makes repeated searches across acceptor sites, OST variants and glycan pathways practical without specialised cell-culture equipment. OpenCFPS™ fits this infrastructure role through 96-well screening and milligram-scale production within the same reagent system. Its documented formulations and lot-level QC address the requirement beneath throughput, namely that differences between wells reflect experimental choices under controlled reagent conditions.
Reagent reproducibility as the practical prerequisite for glycosylation results that transfer from screen to scale
Crude extracts vary in nuclease activity, chaperone composition and energy metabolite levels. Those differences affect both protein yield and the performance of OST enzymes or glycosyltransferases. Occupancy and glycoform distribution are therefore sensitive to composition. A successful screen cannot reliably predict a later production run if the extract changes in ways the workflow does not document.
The plant-cell characterisation provides a concrete example of batch assessment. It reported reproducible glycan profiles across independent lysate batches, while commercial release specifications use eYFP yield as a batch quality indicator. In prokaryotic glycosylation workflows, consistent enrichment of OST or glycosyltransferase components is also necessary, because variable enzyme loading can change glycosylation efficiency independently of the selected target sequence.
OpenCFPS provides published lot-level QC data and fully documented formulations for standardisation and troubleshooting. Those records do not substitute for glycosylation-specific evidence. When a result fails to transfer, the records help separate questions about what is in the extract from questions about OST loading or whether the target is accessible. A scientist who has spent months finding a suitable PglB variant or glycan pathway needs an extract with a record of performance that supports repeating the result next month and moving it from screening to production.
Sources
- Establishing a Cell-Free Glycoprotein Synthesis System for Enzymatic N‑GlcNAcylation
- Glycosylation of Structured Protein Domains in Cell-Free Reaction Environments
- 1 A scalable cell-free manufacturing platform for two-step bioproduction of 1
- ALiCE^®^: A versatile, high yielding and scalable eukaryotic cell-free protein synthesis (CFPS) system