Eukaryotic Versus Prokaryotic Cell-Free Systems for Complex Proteins
Protein complexity, not cost, determines which cell-free system to choose.
Choosing between eukaryotic and prokaryotic cell-free systems for complex proteins is a biological decision before it is a yield or cost decision. The target’s need for post-translational modifications, assisted folding, and membrane integration sets the requirements for the machinery that can make a functional protein. Throughput, price, and reproducibility then distinguish the workable options.
What cell-free protein synthesis is and what distinguishes prokaryotic from eukaryotic systems at the machinery level
Cell-free protein synthesis (CFPS) reproduces cellular protein synthesis in vitro using machinery extracted from cells. Both prokaryotic and eukaryotic systems can start from a DNA or PCR template and complete translation in hours, rather than the days to weeks required by cell-based expression. Their reaction format is not the defining difference. The distinction lies in two inherited features, namely the translational machinery and the capacity for post-translational modification (PTM) and chaperone-assisted folding.
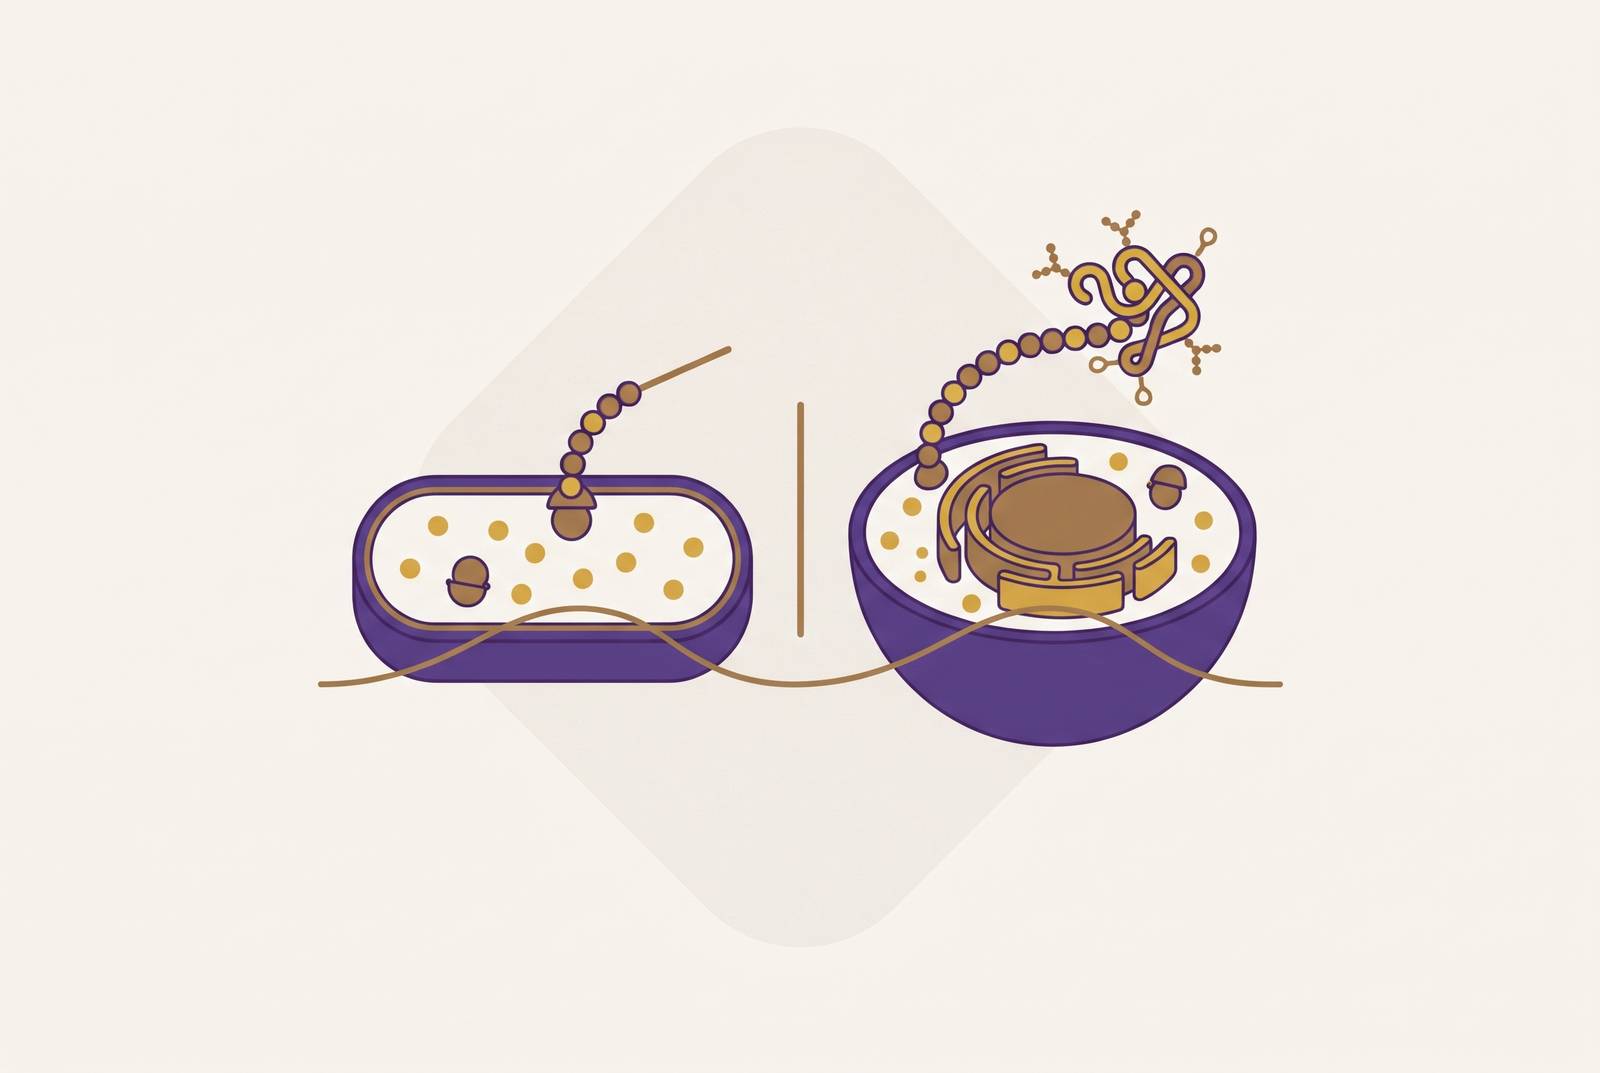
Prokaryotic systems, predominantly based on E. coli lysates, provide efficient, well-understood bacterial translation machinery. They lack the eukaryotic PTM enzymes, chaperone networks, and membrane structures needed for many complex maturation processes. Eukaryotic extracts retain different combinations of these capabilities, including translationally active membrane scaffolds when endoplasmic reticulum-derived microsomal vesicles survive preparation. Their source organisms span mammals, plants, insects, fungi, and protozoa, with different PTM repertoires. Both system types offer an open reaction environment without a living host, but the chassis determines which biological operations that environment can support.
Where prokaryotic systems lead in yield, simplicity, and protein scope
E. coli-based CFPS is the rational first choice for proteins that do not require eukaryotic PTMs or specialized folding assistance. It offers high yield and low cost, is easy to access, and works with automation. Standard reactions can produce hundreds of micrograms to milligrams of protein per milliliter. That output supports both variant screening and production, rather than confining prokaryotic systems to preliminary expression tests. PCR products can also be used directly to express multiple variants at once without cloning or transformation.
Reaction preparation has become less burdensome as well. Lang, Zhang et al. show in a bioRxiv preprint that systematic screening cut the number of essential core reaction components from 35 to 7 while keeping expression at the same level or improving it. Their “fast lysate” protocol also eliminates traditional runoff and dialysis steps. The simplification reduces the number of components requiring preparation and optimization. It addresses a practical barrier that had limited adoption of conventional E. coli CFPS.
The optimized system produced biologically active restriction endonuclease BsaI, assessed by DNA cleavage assay, and vimentin that self-assembled into filaments, assessed by negative-stain electron microscopy. These results extend its scope to strongly cytotoxic and aggregation-prone proteins. Toxicity poses no host-survival constraint because the reaction contains no living cells. The boundary is therefore not whether a protein is challenging, but whether its maturation requires machinery the bacterial extract lacks.
The biological limits of prokaryotic systems in PTMs, disulfide bonds, and chaperone-assisted folding
Standard E. coli CFPS cannot compensate for missing maturation machinery merely by translating more protein. E. coli lacks native protein glycosylation machinery, so an unengineered bacterial extract cannot produce the required glycosylation of a glycoprotein target. Standard systems also lack the eukaryotic machinery for phosphorylation, lipidation, signal peptide cleavage, and membrane integration described here. For targets whose activity, localization, or stability depends on those processes, even abundant translation is not enough.
Disulfide formation presents a different kind of limitation. Low oxidative folding efficiency in bacterial extracts restricts formation of bonds needed by many secreted and extracellular proteins. Redox additives and protein disulfide isomerase (PDI) can partially compensate, making a disulfide-rich but non-glycosylated target a plausible candidate for engineered prokaryotic CFPS. This route needs careful optimization and validation, and success cannot be taken for granted.
Folding assistance is also only partly recoverable through supplementation. Bacterial lysates lack the full eukaryotic chaperone networks that help some multi-domain proteins fold during translation, increasing the likelihood of misfolding or aggregation. Exogenous chaperones can help selected targets, but add components, expense, and experimental work. Vimentin’s successful expression shows what optimization can achieve for an individual aggregation-prone protein. Neither chaperone supplementation nor redox adjustment supplies the missing glycosylation or translocationally active membranes.
What eukaryotic CFPS systems provide and how chassis choice determines available PTMs
An extract from a eukaryotic source may still lack the machinery for the modifications a target needs. The source chassis and retained structures define that capability. A useful comparison must weigh PTM scope, membrane integration, yield, and known gaps together. Systems that perform well on translation may still lack an essential maturation step. The distinction is particularly clear between insect cell and wheat germ extracts.
Stech et al. demonstrate that extracts derived from Spodoptera frugiperda Sf21 cells retain translocationally active, endoplasmic reticulum-derived microsomal vesicles. These provide a natural lipid bilayer for membrane protein embedding and support glycosylation, signal peptide cleavage, lipidation, phosphorylation, and disulfide bond formation. Their continuous-exchange CFPS (CECF) system also produced biologically active human tissue-type plasminogen activator (tPA), which contains multiple intramolecular disulfide bonds. Continuous exchange gives more output than batch operation, but its yields are still generally below prokaryotic batch yields for most proteins.
Wheat germ offers a different balance of capabilities. It is established and high-yielding, making it suitable for non-modified proteins when output is the priority. However, no glycosylation is observed, and phosphorylation is commonly reduced or variable. Its translation performance therefore does not qualify it for glycoproteins or targets that require dependable phosphorylation. Nor does eukaryotic provenance by itself establish the translocationally active membrane support demonstrated in insect extracts.
Membrane proteins as the clearest test case for system selection
Membrane proteins require more than synthesis of a polypeptide chain. Their expression can depend on access to a physical lipid bilayer during translation, together with the machinery that directs integration into it. For this requirement, the decisive distinction is the presence of translocationally active microsomal vesicles. Standard prokaryotic CFPS and eukaryotic extracts without those structures do not supply the necessary machinery. To express a membrane receptor or ion channel that needs co-translational membrane integration, a researcher needs a membrane-competent eukaryotic system.
Insect cell CECF provides a demonstrated route. Its retained vesicles allow newly synthesized proteins to enter vesicle lumens or embed directly into the natural membrane scaffold during translation, supporting topology and activity. This is a physical function.
In cell-based production, toxic or destabilizing membrane proteins can create tension between host viability and protein accumulation. An extract has no host to preserve. Its open environment also permits screening of redox potential, detergent supplementation, lipid composition, and chaperone concentration to adjust folding conditions.
Yield and cost asymmetry between systems and its implications for workflow design
Eukaryotic CFPS typically produces several to tens of micrograms per milliliter in standard batch mode. With that lower output, the strongest reason to use more resources is a protein’s need for the system’s biological machinery. Commercial eukaryotic kits also cost substantially more per reaction than commercially available E. coli systems. Cost therefore compounds the throughput constraint imposed by yield. The practical comparison concerns how much biologically suitable protein a workflow needs.
CECF replenishes substrates and removes inhibitory byproducts over extended reaction times, allowing insect cell systems to exceed their batch-mode output. That makes focused production more viable. The improvement gives researchers a choice of operating mode after they have selected the necessary chassis, with the broader yield asymmetry remaining.
Prokaryotic CFPS favors high-throughput screening across many variants, while eukaryotic CECF favors focused production of validated targets requiring PTMs. Prokaryotic screening followed by eukaryotic expression is appropriate where the initial experiment does not depend on the missing modification. If that modification is essential to the function being tested, the screen itself requires a compatible eukaryotic chassis.
Reproducibility and standardization as distinct vulnerabilities in both system types
Reproducibility remains a consequential weakness across CFPS platforms. Prokaryotic systems vary with extract preparation, DNA templates, and reagent batches, while eukaryotic systems introduce additional variation through retained organelles, lipid vesicles, and diverse PTM machinery. Eukaryotic platforms have consequently remained largely in small-scale research settings, affected by inconsistent PTMs, low yields, limited scalability, and concerns about reproducibility.
Results from different laboratories are hard to compare when studies use different reactor types, reaction compositions, and reaction lengths. A yield reported for one set of conditions does not show how the system will perform under another. Simpler prokaryotic formulations reduce the parameter space requiring characterization, but do not remove the need for it. The seven-component system illustrates how simplification can make control more tractable. It does not make extract identity or reagent quality irrelevant.
Responsible selection therefore includes lot-level lysate quality-control data, documented reaction formulations, and validated workflows specifying mixing geometry, oxygenation, and temperature. These variables need close attention when moving from one reaction format to another. High-throughput plates and bench-top tubes differ in oxygenation and mixing, which can have a large effect on yield. Those effects must be characterized empirically. Well-documented reagents and operating conditions make biological performance easier to reproduce and distinguish from a preparation or handling problem.
A decision framework for matching biological requirements to system capability
The choice of system should start with the modifications the protein needs for its intended function. If glycosylation is essential, an insect cell eukaryotic system with active microsomal vesicles provides the clearest starting point among the options described. Standard prokaryotic CFPS, wheat germ, and rabbit reticulocyte systems do not meet that requirement. Membrane integration or signal peptide cleavage similarly directs selection toward translocationally active membrane structures, with insect cell CECF offering demonstrated performance.
Disulfide bonds call for a more conditional choice. A eukaryotic oxidative folding environment is preferred, but a non-glycosylated target may justify prokaryotic optimization with PDI and redox additives. When phosphorylation is needed, each chassis must be assessed because wheat germ performance is reduced or variable, while insect cell systems generally support it. Bacterial folding assistance is likely to be enough if it can supply the chaperones a target needs. For an aggregation-prone, non-glycosylated protein, optimized prokaryotic CFPS is a rational starting point, with eukaryotic follow-up if folding proves inadequate.
Both system types remove the viability constraint, leaving prokaryotic CFPS as the cost-efficient default when no additional maturation requirement intervenes. Cytosolic proteins without eukaryotic PTM or specialized folding requirements likewise favor optimized bacterial extracts. The BsaI and vimentin results support that broader scope without extending it to glycoproteins or membrane-dependent targets. Difficulty in cell-based expression is not, by itself, evidence of a need for eukaryotic machinery.
Once the workflows meet the protein’s biological needs, the scale of the experiment can guide the choice between them. Many-variant screening favors prokaryotic throughput, while production of PTM-dependent proteins favors eukaryotic CECF. Reagent documentation remains a selection criterion in either case, including lot-level quality control and a formulation matched to the intended reaction format.
Sources
- A simplified and highly efficient cell-free protein synthesis ...
- Eukaryotic cell-free protein synthesis: Chassis diversification, system engineering, and emerging applications - PubMed
- Eukaryotic cell-free protein synthesis: Chassis diversification, system engineering, and emerging applications - ScienceDirect
- A Continuous-Exchange Cell-Free Protein Synthesis System Based on Extracts from Cultured Insect Cells
- A comparative study of protein synthesis in in vitro systems: from the prokaryotic reconstituted to the eukaryotic extract-based
- A simplified and highly efficient cell-free protein synthesis system for prokaryotes